

Our Research

Striatal Interneurons Diversity
The striatum contains a far richer diversity of interneuron types than historically appreciated. Our work has uncovered previously unknown GABAergic interneuron classes each defined by unique physiological, synaptic, and anatomical features. These discoveries revealed that striatal inhibition is not uniform but instead composed of distinct microcircuits with specialised computational roles. By combining transgenic strategies, optogenetics, and high-resolution electrophysiology, we aim to build a refined taxonomy of striatal interneurons and to understand how their diversity supports flexible behaviour.

Main anatomical and electrophysiological characteristics of striatal GABAergic interneurons.


Here, we describe a novel population of striatal GABAergic interneuron (Spontaneously Active Bursty Interneurons, SABIs, Assous et al., 2018) and provide several lines of evidence suggesting that it represents the first interneuron-selective interneuron in striatum. Striatal interneurons and their synaptic connections are suggested to play an important role in the formation of ensembles of striatal SPNs.
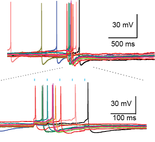
As depicted in the figures, SABIs are spontaneously active and fire in bursts. These interneurons do not significantly innervate SPNs and their inhibition (using optogenetics) induces disinhibitory currents in SPNs suggesting the inhibition of other striatal GABAergic interneurons.
Assous et al., 2018
Tepper et al., 2018

Circuit mapping and connectivity


Our research reveals that striatal interneurons form structured, hierarchical inhibitory networks. Instead of a single, uniform inhibitory pathway onto spiny projection neurons (SPNs), we identified cell-type-specific motifs that govern information flow: selective GIN→SPN pathways, interneuron-selective interneurons, and heterosynaptic interactions such as electrical coupling between THINs and NGFs. We further demonstrated that THINs provide targeted inhibition onto LTS interneurons, adding another layer of hierarchical organisation, and that cholinergic interneurons (CINs) innervate diverse GABAergic interneuron populations, enabling broad, flexible modulation of local circuits. Together, these findings redefine the striatal microcircuit as a multi-layered computational system in which interneuron–interneuron interactions critically sculpt basal ganglia output.

Kocaturk et al., 2022
Assous et al., 2017

Integration of extrinsic afferents


Assous et al., 2019


Assous et al., 2017




Striatal processing is strongly shaped by the identity of its incoming excitatory inputs. Our work demonstrated that cortical, thalamic, and brainstem afferents engage distinct interneuron-defined microcircuits rather than providing uniform excitation. Using a double optogenetic strategy, we showed that parafascicular thalamic (PfN) inputs selectively recruit specific GIN pathways, revealing unexpected disynaptic motifs and disproving the idea of homogeneous thalamostriatal drive. In parallel, our work uncovered a previously unknown glutamatergic projection from the pedunculopontine nucleus (PPN) that evokes powerful disynaptic inhibition of SPNs through targeted interneuron activation and drives behavioural responses in vivo. Together with pathway-specific cortical engagement, these findings establish the striatum as an input-specific integrator in which each afferent source activates a dedicated microcircuit with distinct computational roles.
Linking Defined Circuits to Behaviour


A central goal of our lab is to connect microscale circuitry to behavioural operations. Using silicon-probe electrophysiology, in vivo optogenetics, and calcium imaging, we examine how identified interneuron circuits and specific afferent pathways shape learning, action selection, and cognitive flexibility. By manipulating defined circuit nodes such as CIN-driven inhibition or specific extrinsic afferents, we test mechanistic hypotheses about how striatal computations generate adaptive behaviour. This approach bridges cellular-level discoveries with network-level and behavioural function.
Let’s Work Together
Get in touch so we can start working together.


